For researchers and biotech professionals navigating the rapidly evolving landscape of genome engineering, the choice of editing tool extends far beyond the well-known CRISPR-Cas9 system. While newer technologies garner significant attention, established platforms like Zinc-Finger Nucleases (ZFNs) and Transcription Activator-Like Effector Nucleases (TALENs) maintain critical relevance for specific applications due to their distinct mechanisms and long history of use. Alongside these, advanced CRISPR-based systems like Base Editing offer unprecedented precision for tasks that older methods cannot easily accomplish. The decision to use one of these technologies hinges on fundamental differences in how they target DNA, the type of genetic change required, and the acceptable tolerance for off-target effects. A clear understanding of these trade-offs is essential for designing successful experiments and developing effective next-generation therapeutics.
Introduction to Gene Editing Technologies
The ability to make precise, site-specific modifications to the genome has revolutionized biological and biomedical sciences. Programmable nucleases, including ZFNs, TALENs, and the CRISPR-Cas9 system, have been central to this transformation. These tools generally operate by introducing a targeted double-strand break (DSB) at a specific location in a chromosome. The cell’s own DNA repair machinery is then co-opted to fix this break.
This natural repair process can be guided in one of two ways: through non-homologous end joining (NHEJ), which often introduces small insertions or deletions (indels) that can disable a gene, or through homology-directed repair (HDR), which can use a supplied DNA template to insert new genetic information or correct a faulty sequence. However, a newer class of editors, known as base editors, bypasses the need for a DSB entirely, instead using enzymatic chemistry to directly convert one DNA base to another, offering a more precise method for correcting single-letter mutations.
Zinc-Finger Nucleases (ZFNs): Precision through Protein Engineering
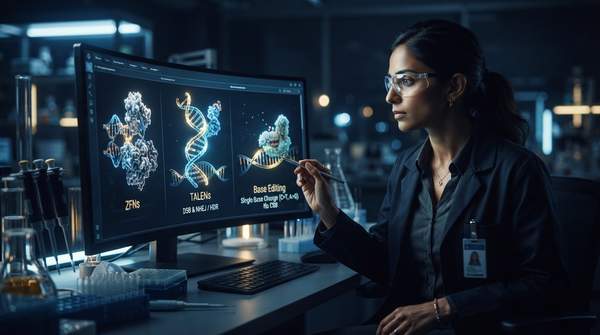
As one of the earliest platforms for targeted genome editing, Zinc-Finger Nucleases rely on a protein-based system for DNA recognition. The targeting component is constructed from a chain of engineered zinc finger proteins, each designed to recognize a specific three-base-pair sequence of DNA. By linking several of these modules together, researchers can build a custom protein that binds to a longer, unique site within the genome. This DNA-binding domain is then fused to a nuclease enzyme called FokI. A key feature of the ZFN mechanism is that the FokI nuclease is only active when two of them come together, or dimerize.
This means two separate ZFNs must bind to opposite strands of the DNA at the target site in a precise orientation to bring the FokI domains together, which then creates the double-strand break. This dimerization requirement significantly enhances the specificity of the edit, reducing the likelihood of cuts at unintended locations.
Transcription Activator-Like Effector Nucleases (TALENs): Modular Design for Targeted Breaks
Similar to ZFNs, Transcription Activator-Like Effector Nucleases are fusion proteins that combine a custom DNA-binding domain with the FokI nuclease to induce a targeted double-strand break. The primary difference lies in the nature of the DNA-binding domain. TALENs are built from Transcription Activator-Like (TAL) effectors, which possess a more straightforward recognition code than zinc fingers. Each TAL effector module recognizes a single DNA base, making the process of engineering a TALEN to target a new sequence more modular and less context-dependent than designing a ZFN. Like ZFNs, TALENs operate in pairs, with each partner binding to one side of the target sequence.
The subsequent dimerization of their FokI nuclease domains is required to cleave the DNA, a feature that provides a crucial layer of specificity. While the engineering is simpler than for ZFNs, TALENs are notably large proteins, which can present challenges for delivery into cells, particularly in therapeutic contexts.
Base Editing: Precise Single-Nucleotide Changes without Double-Strand Breaks
While ZFNs and TALENs excel at creating DSBs to disable genes or insert new ones, many genetic diseases are caused by a single incorrect DNA "letter," or point mutation. Base editing, a technique that leverages the CRISPR system's targeting ability, provides a more precise solution for these cases. According to a review in Nature, base editors use a guide RNA to direct a modified Cas protein to a specific location in the genome. However, instead of cutting the DNA, the Cas protein is catalytically "dead" and functions only as a programmable delivery vehicle.
Fused to this inactive Cas protein is a deaminase enzyme that can perform chemistry directly on a DNA base. This allows the editor to chemically convert one nucleotide into another—for example, changing a cytosine (C) to a thymine (T)—without ever breaking the DNA backbone. By avoiding the DSB, base editing sidesteps the cell's error-prone repair machinery, which can introduce unwanted indels. This makes it a powerful tool for precisely correcting the point mutations underlying many genetic disorders.
Comparative Overview of Gene Editing Technologies
Researchers can use this table as a quick reference to compare the fundamental characteristics, strengths, and weaknesses of ZFNs, TALENs, and Base Editing, aiding in the selection of the most appropriate tool for their specific experimental or therapeutic goals. The table clearly identifies that ZFNs and TALENs are protein-guided tools inducing DSBs for broader genomic modifications with established clinical use, while Base Editing is an RNA-guided tool for precise single-nucleotide changes without DSBs, allowing researchers to match technology capabilities to their specific editing needs.
| Technology | Targeting Mechanism | Type of Edit | Key Advantage | Primary Limitation |
|---|---|---|---|---|
| Zinc-Finger Nucleases (ZFNs) | Engineered zinc finger proteins recognize specific DNA sequences. These proteins are fused to a FokI nuclease, which cuts the DNA upon dimerization. | Creates double-strand breaks (DSBs) repaired by the cell, leading to gene knockouts or insertions. | Proven precision in clinical-grade edits and a long history of use, which can simplify regulatory familiarity. | Complex and time-consuming protein engineering required for each new target site. |
| Transcription Activator-Like Effector Nucleases (TALENs) | Engineered TAL effector proteins recognize specific DNA sequences. Like ZFNs, they are fused to a FokI nuclease that cuts DNA upon dimerization. | Creates double-strand breaks (DSBs) repaired by the cell, enabling gene knockouts or insertions. | High specificity and a more straightforward modular design for protein engineering compared to ZFNs. | Large size can make delivery into cells challenging; still requires significant protein engineering. |
| Base Editing | A guide RNA (gRNA) directs a catalytically impaired Cas protein fused to a deaminase enzyme to a specific DNA location. | Directly converts one DNA base to another (e.g., C to T) without creating a double-strand break. | High precision for correcting point mutations while avoiding the error-prone repair pathways associated with DSBs. | Limited to specific types of single-base changes; potential for off-target edits on nearby bases. |
Choosing the Right Tool: Applications and Trade-offs
Despite the dominance of CRISPR-based systems, ZFNs and TALENs retain significant advantages for certain applications. According to an analysis from Crown Bioscience, their protein-based targeting can make them less prone to off-target effects compared to some RNA-guided systems. Their extensive history means they have been used in clinical-grade edits for genetic disorders like HIV and hemophilia, leading to greater regulatory familiarity. This proven track record makes them a preferred choice for researchers requiring meticulous control, such as in the development of stable cell lines for biomanufacturing. In these contexts, the initial investment in protein engineering is justified by the high fidelity and reliability of the resulting edit.
Conversely, for therapeutic applications aimed at correcting single-nucleotide mutations, base editing offers a clear advantage. The ability to make precise C-to-T or A-to-G conversions without inducing a DSB is a powerful capability. This avoids the generation of indels, which are a common and often undesirable byproduct of DSB-based editing. Both CRISPR-Cas9 and base editing have been used to treat diseases in people, but their strengths lie in different areas. As noted by Nature, CRISPR-Cas9 excels when the goal is to abolish a gene's function by inducing an error-prone repair. Base editing, however, is the more precise tool when the goal is to fix a specific genetic "typo" without otherwise disturbing the genomic sequence.
Selecting the Optimal Gene Editing Tool
Researchers should select a gene editing technology based on the specific type of genetic modification required (e.g., single-nucleotide change vs. gene knockout), the desired level of precision, and the tolerance for potential off-target effects or indel formation. For applications like creating stable cell lines or when regulatory familiarity is a priority, the proven track records and high specificity of ZFNs and TALENs make them strong contenders. The upfront effort of protein engineering is often rewarded with a highly specific and reliable tool. However, if the primary goal is to correct a single-point mutation with minimal disruption to the surrounding DNA, the precision of base editing is unparalleled. It avoids the unpredictable outcomes of DSB repair, making it a superior choice for many therapeutic applications.
The continued relevance of ZFNs and TALENs alongside the rise of advanced CRISPR-based systems underscores a key principle in biotechnology: there is no single "best" editor, only the most appropriate one for a given task. Successful experimental outcomes, such as the precise correction of a point mutation without unintended indels, or the stable integration of a gene in a cell line, will indicate an appropriate technology choice.
Sources
- Bigger than CRISPR? A guide to the latest genome editors — NATURE
- Recent advances in the use of ZFN-mediated gene editing for human gene therapy — BioInsights Publishing
- Advances in CRISPR Base Editing: From Molecular Evolution to Therapeutic Applications in Genomic Medicine - PMC
- GAJ LAB
- Comparing Gene Editing Platforms: CRISPR vs. Traditional Methods — BLOG